INTRODUCTION
One area of major advancement in helminthology has been in understanding genetic and molecular parameters of parasite populations. To a large extent, this progress follows significant developments of molecular markers that are widely used mainly in two fields. Firstly, the study of the genetic evolution of a species and the examination of its taxonomic relationships with other organisms have both been tackled. Secondly, ecology was contracted to identify an organism, investigate population genetics or to consider its dynamic activity within a given environment (Monis et al. Reference Monis, Andrews and Saint2002). Due to the important veterinary and medical significance of cestodes, efficient molecular tools have been explored for many species to improve detection, prevention and management of zoonotic transmission in particular (Yang et al. Reference Yang, Rosenzvit, Zhang, Zhang and McManus2005; Smith, Reference Smith2009). Echinococcus multilocularis is the causative agent of the human alveolar echinococcosis (AE), and is one of the most threatening parasitic zoonoses of the Northern hemisphere. Its transmission pattern involves different mammalian hosts. Foxes (Vulpes vulpes) and dogs (Canis lupus familiaris) act as the main definitive hosts (DH). A wide range of small-mammals, including mainly rodents such as Arvicola spp. and Microtus spp. and Lagomorpha of the genus Ochotona act as intermediate hosts (IH) (Vuitton et al. Reference Vuitton, Zhou, Bresson-Hadni, Wang, Piarroux, Raoul and Giraudoux2003). Cystic echinococcosis (CE) is a widespread and severe zoonosis caused by infection with the larval stage of Echinococcus granulosus sensu lato (E. granulosus s.l.). As with AE, humans acquire CE infections by ingesting Echinococcus eggs via contaminated food or water, through close physical contacts with DH, or directly with faeces of these hosts. Its transmission pattern also involves different mammalian hosts, mainly canids as DH and a large variety of livestock animals as IH. Based on mitochondrial DNA studies, the classification within the E. granulosus s.l. paraphyletic taxon has undergone, and continues to undergo, important changes. E. granulosus s.l. is composed of heterogeneous groups of variants, defined as ‘strains’ (G1 to G10) (Bowles et al. Reference Bowles, Blair and McManus1992; Bowles and McManus, Reference Bowles and McManus1993; Scott et al. Reference Scott, Stefaniak, Pawlowski and McManus1997; Lavikainen et al. Reference Lavikainen, Lehtinen, Meri, Hirvela-Koski and Meri2003). However, these strains are now reorganized within distinct species (Thompson and McManus, Reference Thompson, McManus, Eckert, Gemmell, Meslin and Pawlowski2002; Lavikainen et al. Reference Lavikainen, Lehtinen, Meri, Hirvela-Koski and Meri2003; Nakao et al. Reference Nakao, McManus, Schantz, Craig and Ito2007). E. granulosus sensu stricto (E. granulosus s.s.) encompasses the G1, G2 and G3 strains, E. equinus corresponds to the G4 strain, and E. ortleppi comprises the G5 strain. The G6, G7, G8, G9 and G10 strains have also been classified under a well-supported monophyletic species, E. canadensis (Nakao et al. Reference Nakao, McManus, Schantz, Craig and Ito2007). Moreover, this revised classification seems to be more in accordance with nuclear studies, which emphasizes smaller differences than observed in mtDNA studies among the E. granulosus s.l. stains (Saarma et al. Reference Saarma, Jogisalu, Moks, Varcasia, Lavikainen, Oksanen, Simsek, Andresiuk, Denegri, Gonzalez, Ferrer, Garate, Rinaldi and Maravilla2009).
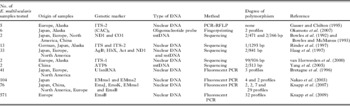
Molecular tools are required to better understand taxonomic relationships between Echinococcus species and infra-specific taxa, as well as to precise molecular tracking of Echinococcus isolates collected from humans and animals based upon geographically or biologically relevant markers. However, so far, molecular studies have exhibited very little genetic variation within E. multilocularis. Notwithstanding the methods used, most molecular markers lacked of discriminatory power. In order to increase the level of resolution and sensitivity of the tools, we set up an original molecular target represented by a highly tandemly repeated microsatellite, called EmsB. In contrast to classical microsatellite targets, PCR amplification of EmsB provided a multi-peak profile, characterized by tandemly repeated microsatellite sequences. This aspect confers to EmsB a higher discriminatory power than all of the currently available molecular tools (see Table 1).
Principal molecular markers used for the genotyping of E. multilocularis from the literature. From Bart et al. 2003 and updated in this present paper

The present paper reviews the different steps which have led to the discovery, characterization and application of this original molecular tool for the evaluation of genetic polymorphism in E. multilocularis and E. granulosus s.l. Its application in several molecular epidemiological studies has suggested new hypotheses on the dispersion pattern of E. multilocularis in endemic foci, especially in the European focus, controversially described as a centrally (Alpine arch area) historical endemic area, and in its peripheries as newly endemic zones (Eckert et al. Reference Eckert, Conraths and Tackmann2000). It also provided new insights in the molecular epidemiology of E. granulosus s.l. and in the demonstration of cross-fertilization between the new defined species of E. granulosus s.s. and E. ortleppi.
THE NEED FOR HIGHLY POLYMORPHIC MARKERS WITHIN THE GENUS ECHINOCOCCUS
Despite substantial efforts to develop and apply valuable genetic tools for E. multilocularis genotyping (Table 1) (Bowles et al. Reference Bowles, Blair and McManus1992; Bowles and McManus, Reference Bowles and McManus1993; Gasser and Chilton, Reference Gasser and Chilton1995; Bretagne et al. Reference Bretagne, Assouline, Vidaud, Houin and Vidaud1996; Haag et al. Reference Haag, Zaha, Araujo and Gottstein1997; Rinder et al. Reference Rinder, Rausch, Takahashi, Kopp, Thomschke and Loscher1997; van Herwerden et al. Reference van Herwerden, Gasser and Blair2000; Nakao et al. Reference Nakao, Sako and Ito2003; Yang et al. Reference Yang, Rosenzvit, Zhang, Zhang and McManus2005; Knapp et al. Reference Knapp, Bart, Glowatzki, Ito, Gerard, Maillard, Piarroux and Gottstein2007; Okamoto et al. Reference Okamoto, Oku, Kurosawa and Kamiya2007), a high discriminatory power was not really achieved except when using microsatellite targets. Overall, an important homology was described within the species E. multilocularis, which could probably be explained first by an almost unique reproduction pattern at the adult stage by homogamy (Haag et al. Reference Haag, Zaha, Araujo and Gottstein1997, Reference Haag, Araujo, Gottstein and Zaha1998) and secondly by the recent report of E. multilocularis and the evolutionary history of the genus (Bowles and McManus, Reference Bowles and McManus1993). It was necessary to search for rapidly evolving DNA fragments. The first study devoted to E. multilocularis genotyping using microsatellite considered the U1 snRNA multi-gene, tandemly repeated in DNA (around 50 copies in the Eukaryote genome), separated by a pentameric microsatellite (Bretagne et al. Reference Bretagne, Robert, Vidaud, Goossens and Houin1991). Analysing samples from North America, Japan and Europe, three profiles were described (a profile was described as a series of peaks on the electropherogram). A regional polymorphism was described and similar profiles were found between North America and Japan, suggesting a putative common origin of E. multilocularis (Bretagne et al. Reference Bretagne, Assouline, Vidaud, Houin and Vidaud1996). The second study focused on 2 single-locus microsatellites, EMms1 (GenBank Access No. AB100031, composed of an array of different triplets) and EMms2 (AB100032 composed of one motif (CAC)n) (Nakao et al. Reference Nakao, Sako and Ito2003). These two microsatellites were used with worms originating from the endemic island of Hokkaido, Japan. Four genotypes were described for EMms1 and two for EMms2. Mixed infections in foxes were also found (worm burdens contained parasites of different genotypes). Unfortunately and in spite of a high level of genetic diversity, it was not possible to link the E. multilocularis allelic frequency to geographical position of foxes, due to the insular origin of samples. In comparison with E. multilocularis, E. granulosus s.l. is less monomorphic and sequencing of some mitochondrial and nuclear DNA targets revealed important genetic diversity, leading to the definition of the above mentioned strains and new species. However, mitochondrial and nuclear markers were not sufficiently polymorphic to identify genetic variations that reflect regional or focal population characteristics. To date, only four single-locus microsatellites have been used to assess E. granulosus s.l. genetic diversity: U1snRNA, EgmSca1, EgmSca2 and EgmSga1. The U1snRNA gene provided 11 distinct profiles among species: 8 for E. granulosus s.s. (G1/G2), 2 for E. ortleppi (G5) and 1 for E. canadensis (G6) (Roratto et al. Reference Roratto, Bartholomei-Santos, Gutierrez, Kamenetzky, Rosenzvit and Zaha2006), but no spatial correlation was observed. Among the three microsatellites described in Bartholomei-Santos and co-workers (Bartholomei-Santos et al. Reference Bartholomei-Santos, Heinzelmann, Oliveira, Chemale, Gutierrez, Kamenetzky, Haag and Zaha2003), only EgmSca1 provided results indicating a weak spatial correlation in 73 Brazilian and Argentinean samples.
ISOLATION AND CHARACTERISATION OF EmsB
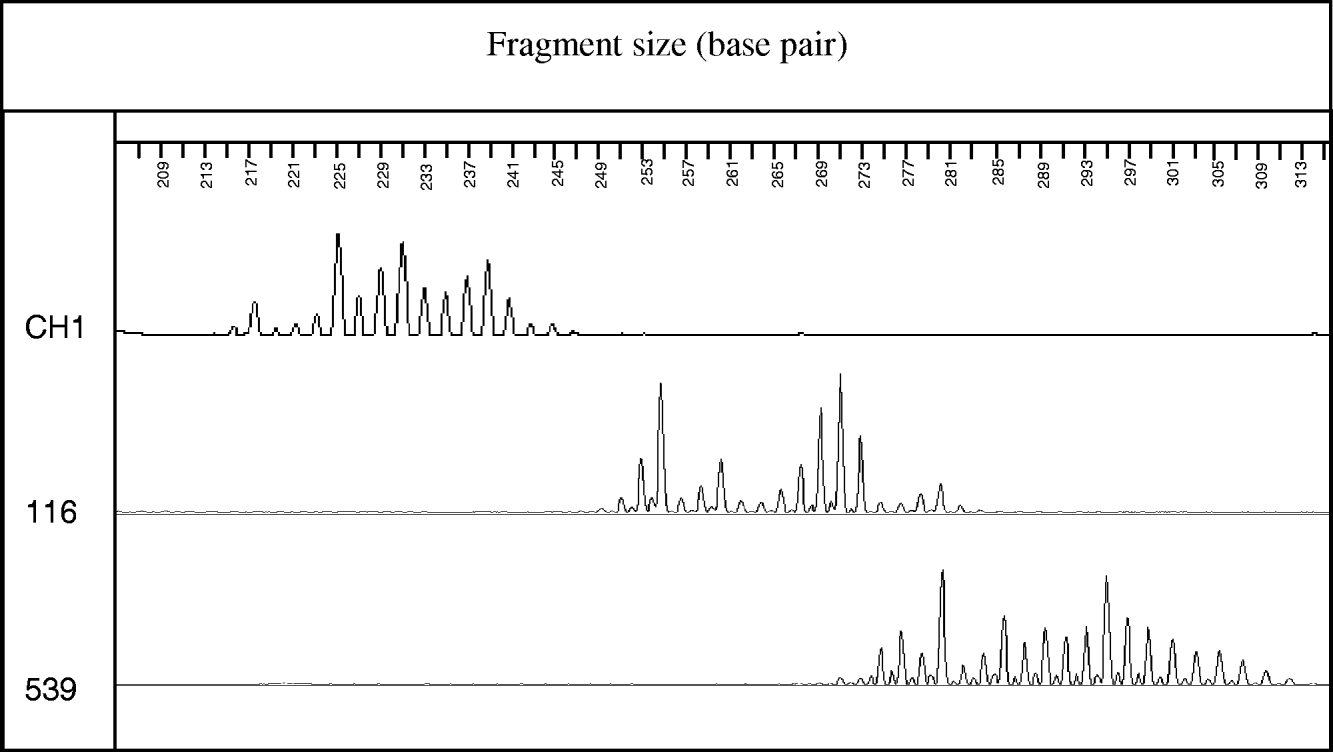
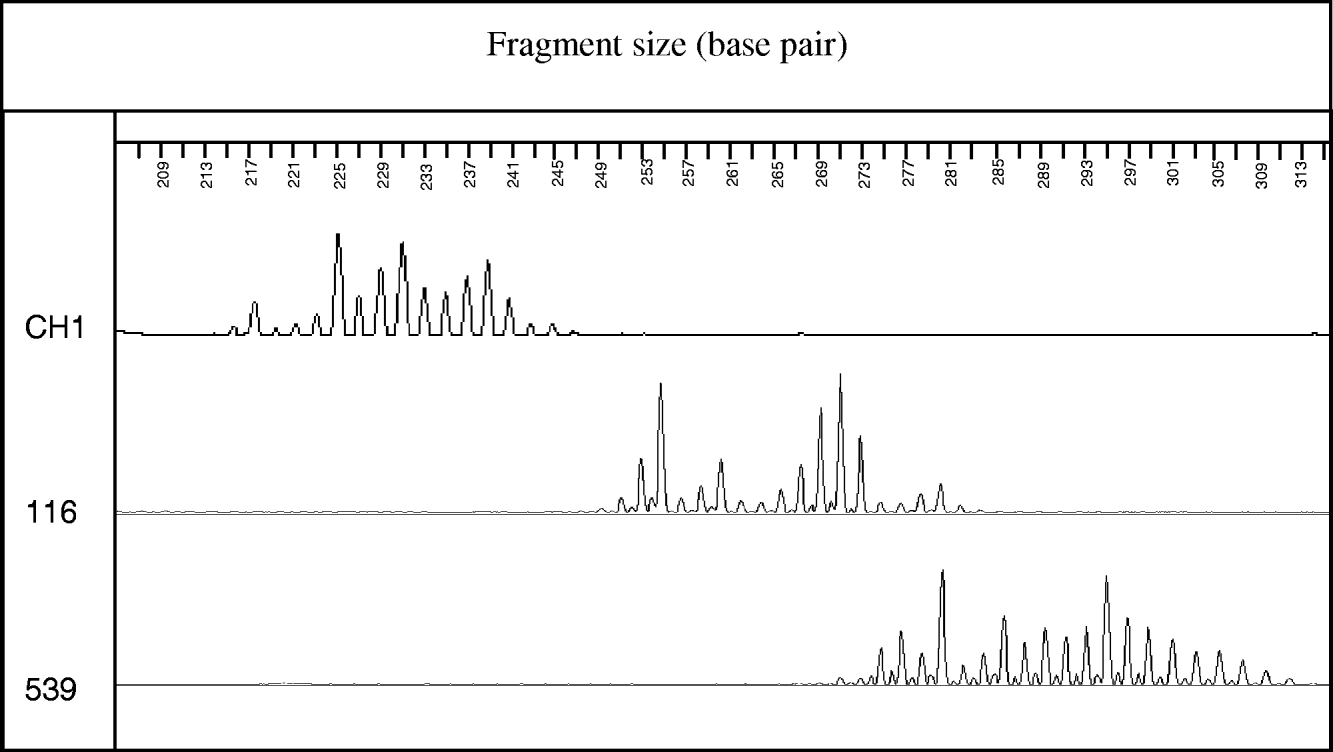
The search for highly polymorphic markers was continued and targeted on new microsatellite sequences that would meet the expected level of discriminatory sensitivity (Bart et al. Reference Bart, Abdukader, Zhang, Lin, Wang, Nakao, Ito, Craig, Piarroux, Vuitton and Wen2006a). After screening an E. granulosus DNA library, 17 microsatellites were identified. This species was used because, at that time, only protoscoleces obtained from hydatid cysts yielded high quantities of pure material without host DNA contamination. From a first inter-species screening, 3 microsatellite targets were found to be polymorphic: EmsJ (GenBank ref. No. AY680845) presenting a repeated motif (CT)n, EmsK (GenBank ref. No. AY680857) with a repeated motif (CA)n and EmsB with two repeated motifs (CA)n (GA)m (n and m, number of repetitions). In comparison to the other microsatellites, EmsB presented a peculiar electropherogram profile, with a notable difference among Echinococcus species and isolates tested (Fig. 1). Based on this finding it was decided to unravel the genetic structure of EmsB in order to explain its non-conventional profile.
Fragment size analyses of the EmsB target, realized on DNA samples of E. multilocularis from Switzerland (CH1), E. canadensis (116), from Mauritania and E. granulosus sensu stricto (539), from Algeria, with the ABI Prism 3100 sequencer.
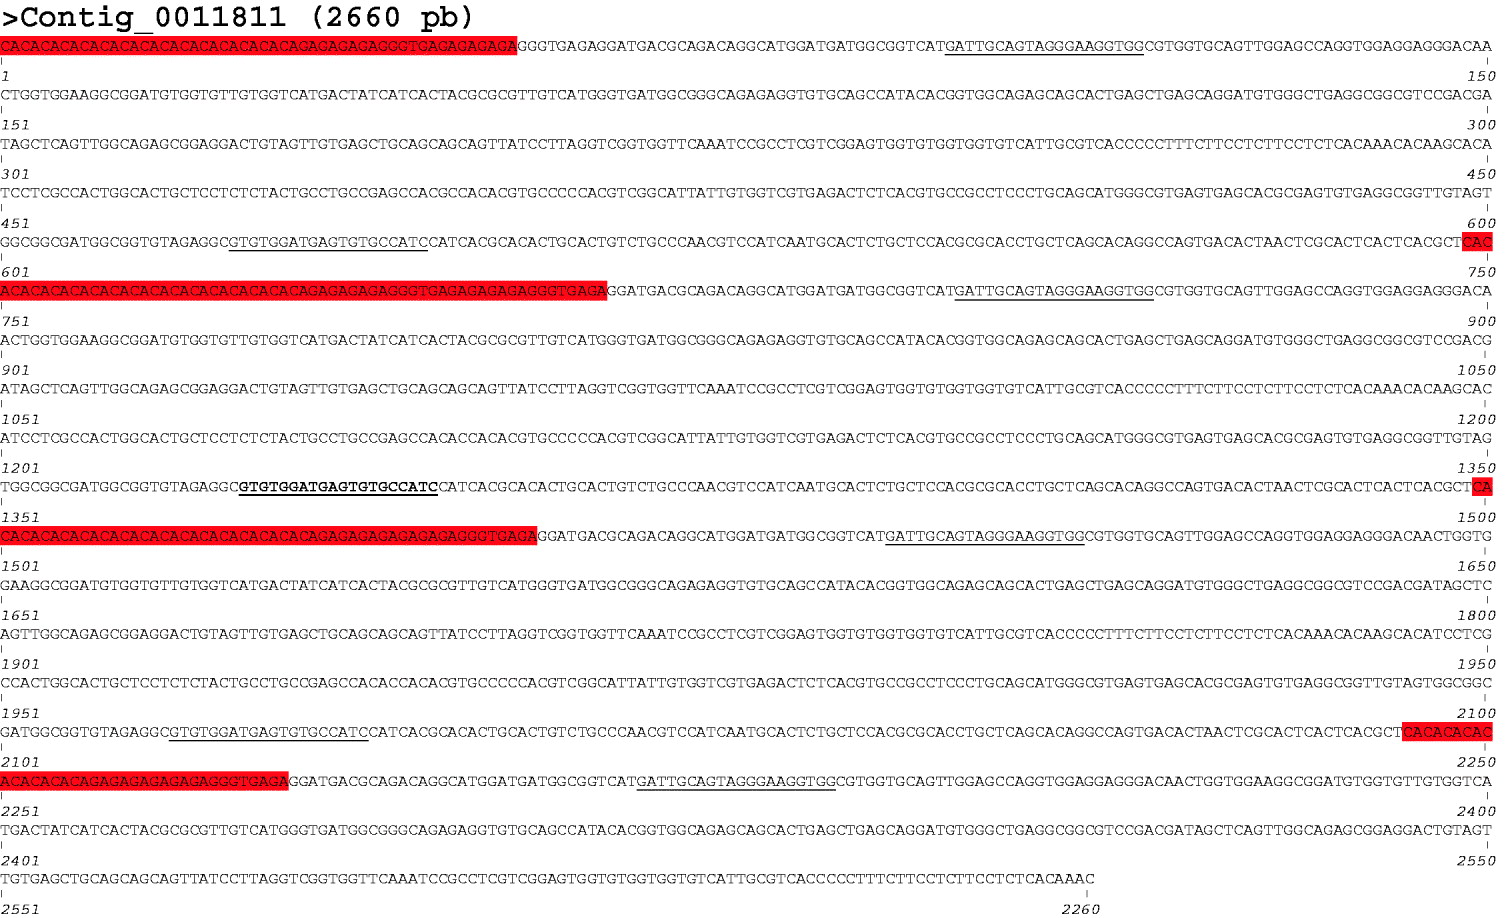
The strategy to elucidate the nature of the multi-peak electropherogram was to isolate by cloning the EmsB PCR products. The screening of 110 clones and analyses of the fragment sizes of each inserted PCR product allowed us to observe single peaks, discarding a possible in vitro slippage of the polymerase during the PCR. The reconstitution of an EmsB profile by addition of the isolated peaks yielded a profile similar to the original one. The sequencing of isolated fragments showed a slight homoplasy phenomenon among fragments of the same size which could be interpreted as an inner polymorphism between the different loci. This phenomenon leads to a loss of information, but the highest level of data provided by a multi-locus marker could easily compensate for this problem (Estoup et al. Reference Estoup, Jarne and Cornuet2002). The complex electropherogram profile of the EmsB target could be due to its presence in multi-copies in the Echinococcus DNA and not to an artefact. This hypothesis was confirmed by quantitative PCR and the number of copies of EmsB was evaluated at 104 copies in the Echinococcus genome (Fig. 2).
Sequence no. 11811 of 2660 bp published in the E. multilocularis Genome Project by the Sanger Institute presenting 4 microsatellite EmsB sequences found tandemly repeated. Repeated motifs are highlighted in red and forward/reverse primers are in green. For the first microsatellite (position 1 to 115 bp), only the reverse primer was found.
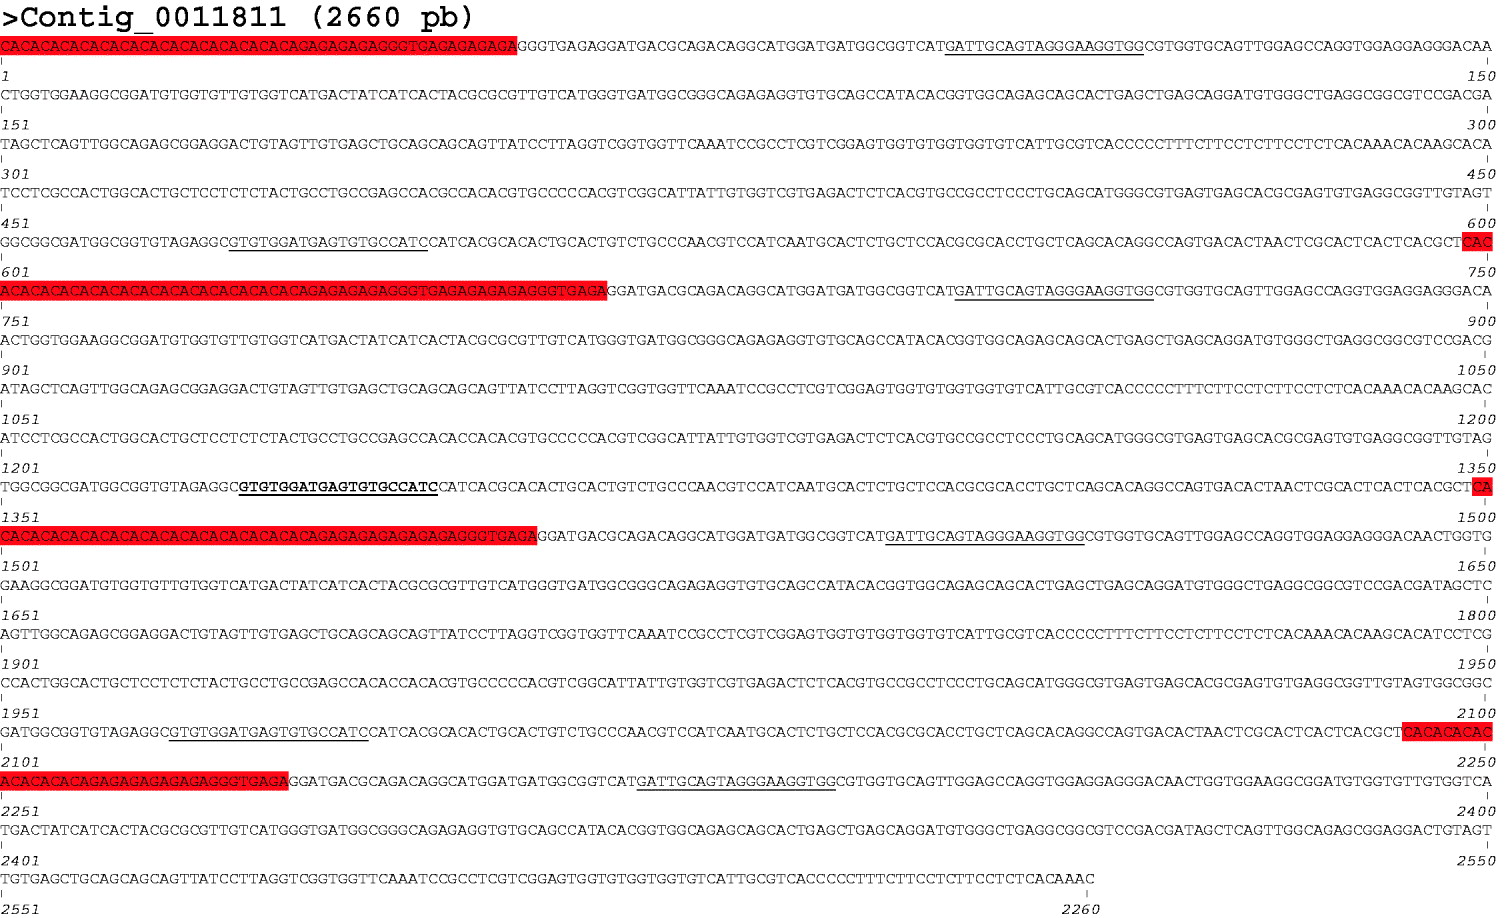
To assess the distribution of this microsatellite in the genome, PCRs with large elongation steps and different primer sets were performed. Several bands, regularly spaced were amplified, that suggested a tandem repetition of the target. The presence of EmsJ, EmsK and EmsB was searched in the recently published genome sequence for E. multilocularis from the Sanger Institute in the framework of the Echinococcus Genome project (http://www.sanger.ac.uk/Projects/Echinococcus). EmsJ and EmsK were found in a single copy in the E. multilocularis data base, in the contig sequences No. 4805 and 18680 respectively. EmsB was found among several short contig sequences and for some of them tandemly repeated (e.g. contig No. 11811 where EmsB A/C was found 4 times (Fig. 2) and contig No. 19011, 2 times (data not shown)).
The EmsB PCR products could be characterized by fragment size analyses. Electropherograms revealed a series of peaks, which were called EmsB profiles. Two parameters on the electropherogram were retained to characterize each EmsB profile: the size (in base pairs) of the amplified fragments and the number of targets of the same size were revealed by the intensity of the peaks. The Euclidian distances between two computed profiles could be calculated in order to assess the similarity/dissimilarity among a sample collection. The hierarchical clustering analysis using an unweighted-pair group method and average linkage (UPGMA) (Legendre and Legendre, Reference Legendre and Legendre1998) yielded dendrograms graphically representing the relationships among samples; the robustness was tested by bootstrap resampling.
To complete the characterization of EmsB, stability in time of the microsatellite, reproducibility, repeatability, sensitivity and specificity of its amplification by PCR were all assessed. For stability, three isolates from the E. multilocularis strain F AUB-2, maintained one year in vivo in Meriones unguiculatus were analysed at three different times. The three profiles were highly similar and used to define a genetic distance threshold that discriminates the EmsB profiles. This genetic distance was further used for all the epidemiological surveys performed with EmsB. For reproducibility and repeatability, different DNA polymerases and different conditions of amplification were tested. Reproducibility and repeatability were also tested in different laboratories and by different operators and have provided valid results (Bart et al. Reference Bart, Knapp, Gottstein, El-Garch, Giraudoux, Glowatzki, Berthoud, Maillard and Piarroux2006b). The sensitivity was described on agarose gel with 1 fg of DNA. The specificity was tested on host DNA (human, and mouse (Bart et al. Reference Bart, Knapp, Gottstein, El-Garch, Giraudoux, Glowatzki, Berthoud, Maillard and Piarroux2006b), foxes (Knapp, Reference Knapp2008)) and on a panel of helminths (Casulli et al. Reference Casulli, Bart, Knapp, La Rosa, Dusher, Gottstein, Di Cerbo, Manfredi, Genchi, Piarroux and Pozio2009). Only isolates from the genus Echinococcus yielded appropriate amplifications.
FROM GENOME TO FIELD STUDIES
The usefulness of EmsB to study the genetic diversity of E. multilocularis and E. granulosus with a multi-scale approach was assessed. Three main questions needed to be addressed: (1) Is the polymorphism of the marker sufficient to obtain a molecular signature to recognised ‘strain’ circulating among hosts, without over-discrimination and independent to hosts? (2) What are the geographical limits of its genetic discrimination? (3) Is the marker useful to study the spatial structure and the dynamic activity of the parasite at different geographical ranges/levels?
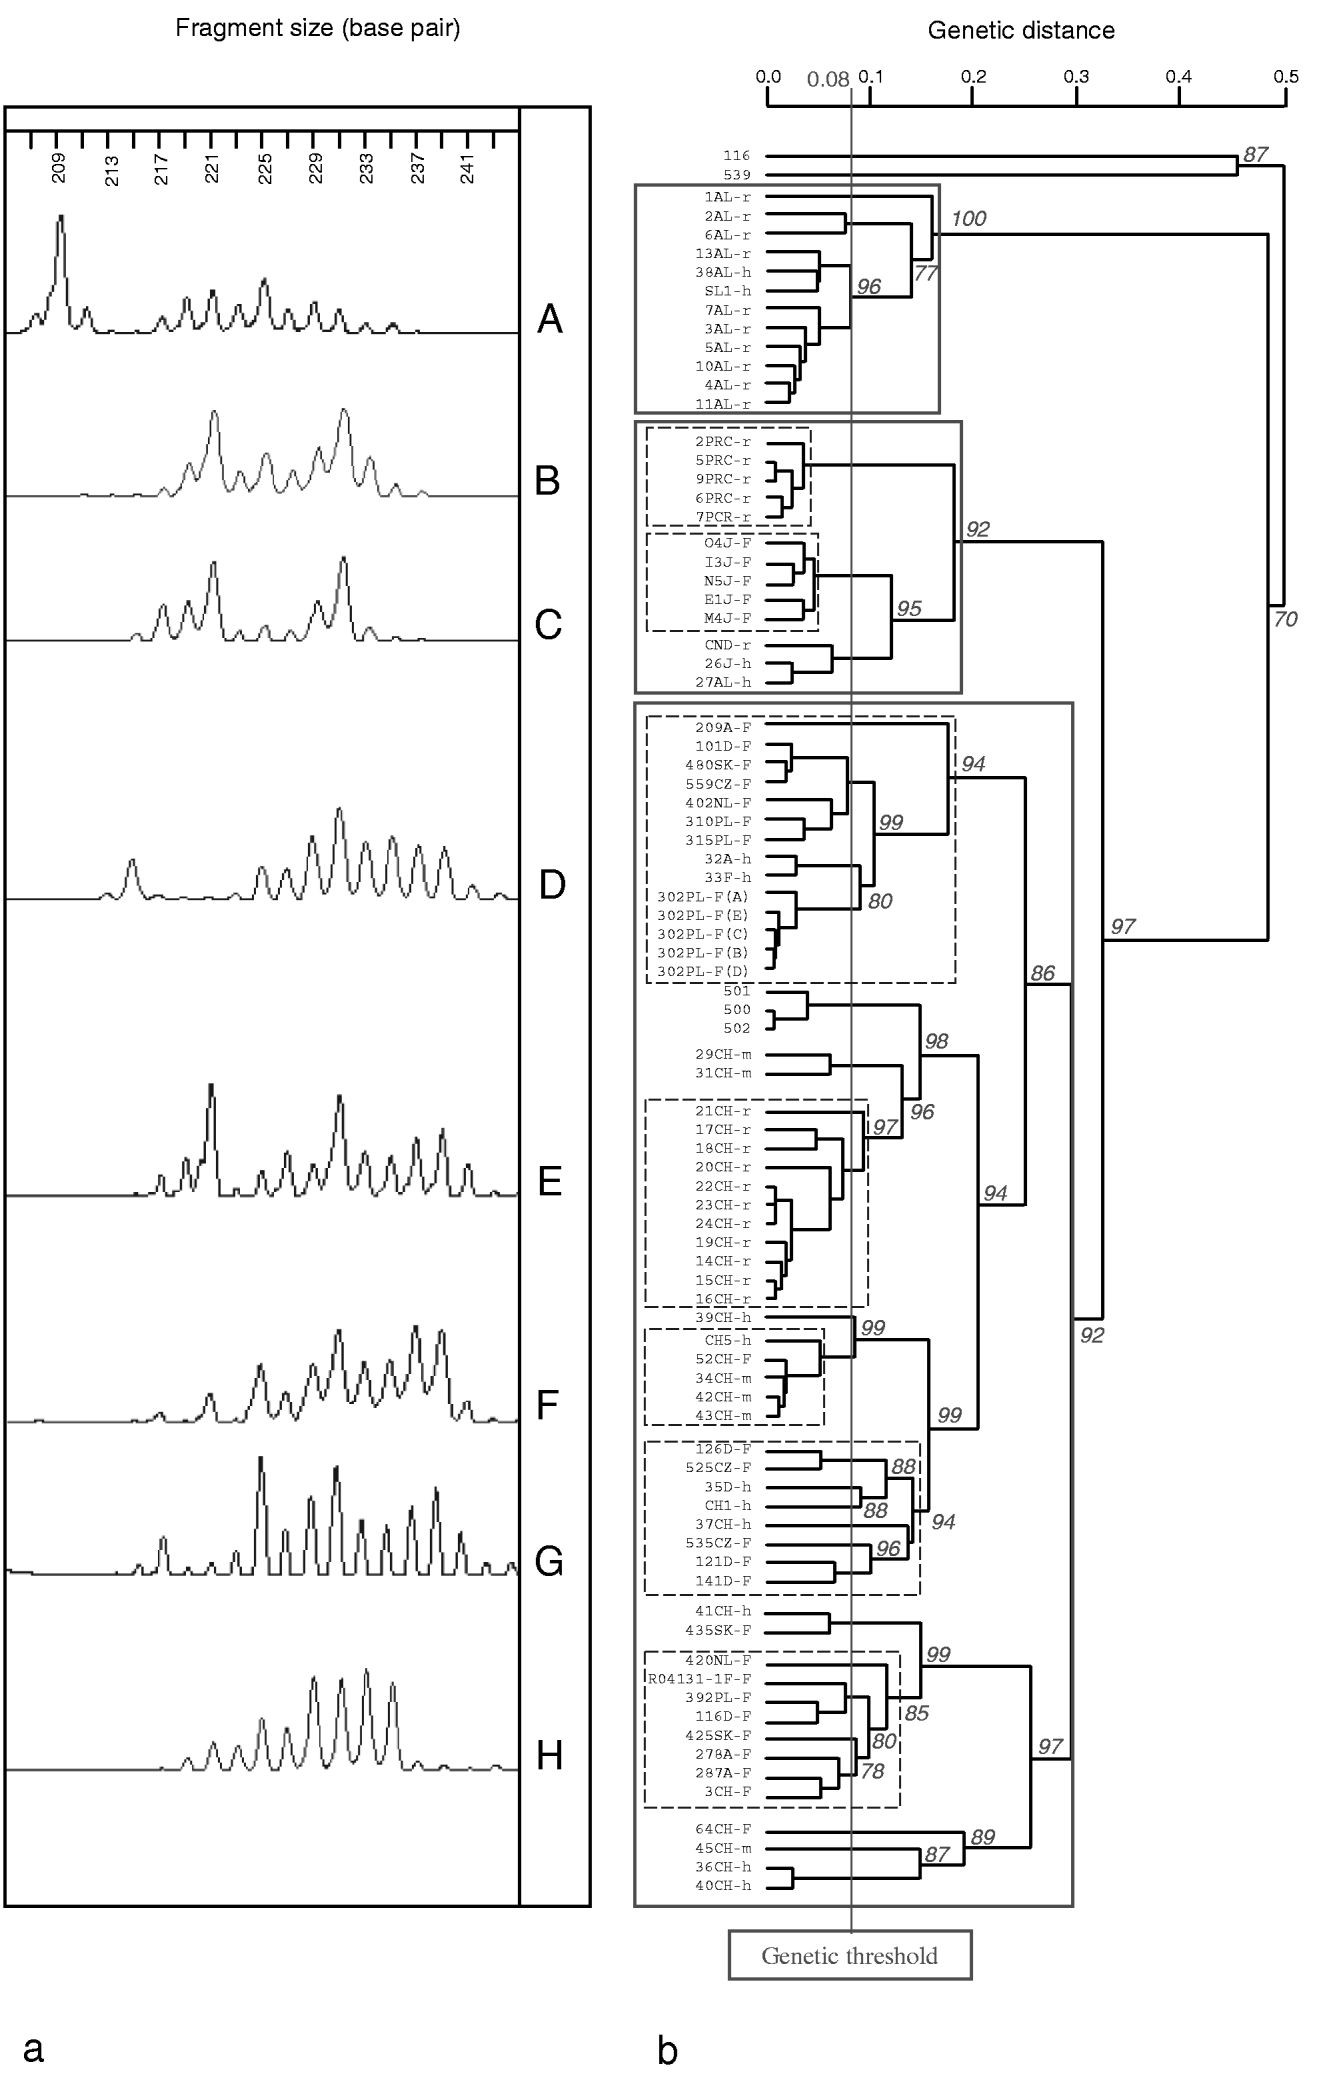
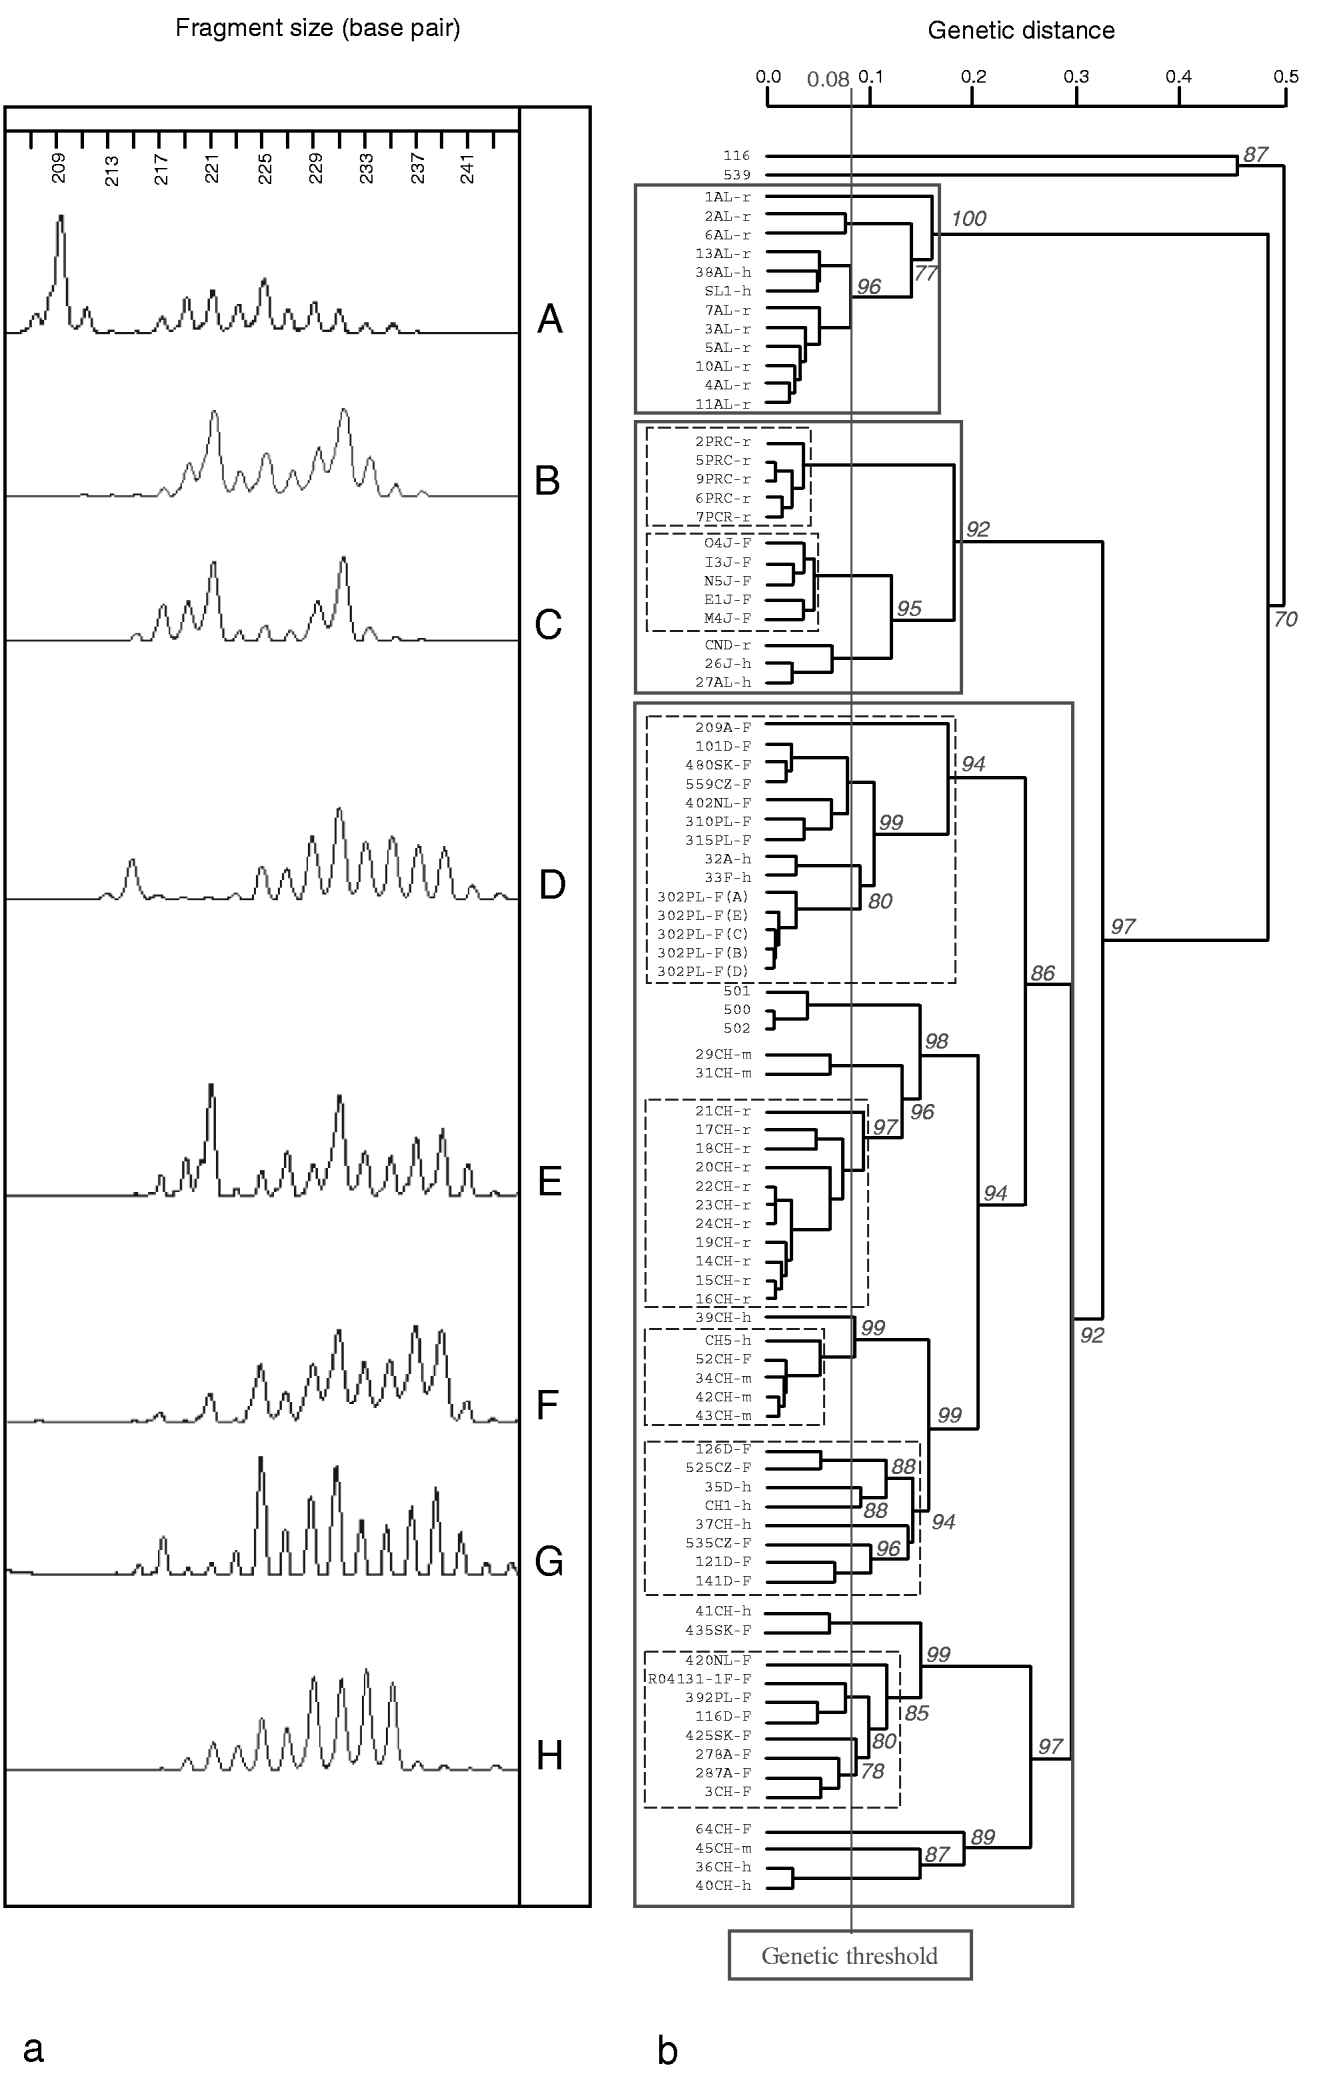
The power of the EmsB marker in the search for E. multilocularis genetic polymorphism was realized with a global collection composed of 76 isolates from humans, monkeys, rodents and foxes, originating from North America (Saint Lawrence island in Alaska and Canada), China (Tibetan plateau), Japan (Hokkaido island) and Europe (Switzerland, France, Germany, Austria, Poland, Czech Republic, Slovakia and the Netherlands) (Knapp et al. Reference Knapp, Bart, Glowatzki, Ito, Gerard, Maillard, Piarroux and Gottstein2007). Finally with the EmsB marker, 29 genotypes were described (Fig. 3) and regional groups (European, North American, Chinese and Japanese groups) were graphically defined, including 23 clusters among the European samples. Same EmsB profiles were found shared as well among DH (foxes) as among IH (humans and monkeys). This finding underlined the independence of EmsB profiles for hosts. To the best of our knowledge, this paper related the highest genetic diversity described for E. multilocularis on a worldwide panel. These findings lead us to believe that EmsB could be employed to retrieve the genetic diversity of individual worms and study the distribution of its genetic variability at different spatial ranges, independent of hosts and investigate the transmission activity of the parasite.
FIELD STUDIES
Further investigations targeted the E. multilocularis genetic diversity with a multi-geographical-scale approach. In order to assess the genetic discrimination threshold of the marker EmsB and its power to describe circulation of the parasite among different host populations, three geographical scales were investigated: (1) at a regional scale approach, taking into consideration the interaction of several fox populations; (2) at two local scale approaches (territory of a fox population), in two different topographical situations, first in an undulating area in the French Ardennes (North of France) and in a mountain area in the Val Pusteria (North of Italy); and finally (3) at a micro-local scale, by investigating parasites isolated from close related rodent hosts, collected in a very limited field (around 100 m2) in Switzerland and independently in Alaska, to assess the limits of the EmsB discrimination power for closely related samples.
THE ECHINORISK PROJECT: EmsB STUDY TO ADDRESS THE GENETIC DIVERSITY OF E. MULTILOCULARIS AT THE CONTINENTAL SCALE IN EUROPE
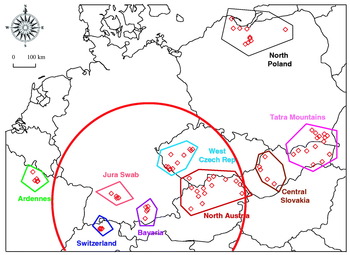
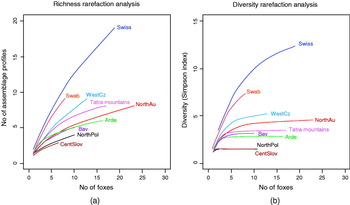
In Europe, E. multilocularis is historically described as predominantly occurring on the North side of the Alpine arch (East of France, South Germany, Austria and Switzerland), essentially because most of human records are described in this area (Eckert et al. Reference Eckert, Conraths and Tackmann2000; Kern et al. Reference Kern, Bardonnet, Renner, Auer, Pawlowski, Ammann and Vuitton2003). In order to study the pattern of occurrence E. multilocularis in Europe, a collection of 571 adult worms from 123 geo-referenced foxes (Fig. 4) were sampled in 9 European regions, including the historical core (Switzerland, North Austria, Germany (Swabian Jura and Bavaria) and West Czech Republic) and 4 areas considered as newly endemic regions (North of France, Central Slovakia, Tatra mountains and North Poland) (Knapp et al. Reference Knapp, Bart, Giraudoux, Glowatzki, Breyer, Raoul, Deplazes, Duscher, Martinek, Dubinsky, Guislain, Cliquet, Romig, Malczewski, Gottstein and Piarroux2009). This study described a total of 32 EmsB profiles. Among them, six profiles represented 69% of the whole sample collection and 5 of them were widely described in the European territory surveyed. The sampling effort was tested by a rarefaction analysis (Colwell, Reference Colwell2005) showed that the genetic richness was not reached in almost all studied sub-regions (Fig. 5). However, the genetic diversity was found to be higher in the historical endemic area compared to peripheral zones. Moreover, in each peripheral zone, one profile was found to be dominant. This profile was also found in the historically endemic area but was harboured by only a few specimens. This finding prompted the occurrence of a founder event, where a numerically low represented species or a genotype exported to a hitherto free territory could be found dominant after colonization, followed by its spreading (Templeton, Reference Templeton2008). Distinctive features of local parasite cycles, e.g. involvement of peculiar intermediate hosts, landscapes or effect of human behaviours (agriculture, deforestation, occupation of fox territory, etc.) could also have an important role in the parasite genotype distribution into the environment as it was suspected in the French Ardennes region (Knapp et al. Reference Knapp, Guislain, Bart, Raoul, Gottstein, Giraudoux and Piarroux2008). Overall, findings suggest that the dispersion pattern of E. multilocularis in the endemic European focus could be attributed to a mainland-island spreading and dominant genotypes in peripheral regions of the historical area explained by founder events. Regarding the slow dispersion of the parasite in Europe (Takumi et al. Reference Takumi, de Vries, Chu, Mulder, Teunis and van der Giessen2008), this phenomenon had certainly required longer time than previously reported.
E. multilocularis genetic classification according to EmsB results. On the left side (a), example of electropherograms of EmsB loci (209 bp to 241 bp), using the automatic sequencer ABI Prism 3100™. On the right side (b), dendrogram based on EmsB genotypic data, constructed by hierarchical clustering analysis (Euclidian distance, average link clustering method), with pvclust, under R Project. The approximately unbiased P values (numbers on nodes, in percent) were calculated with a multiscale bootstrap (B=1000). The three solid-line boxes show St. Lawrence Island's samples (upper box), the Asian-North American samples (middle box) and the European samples (lower box). The electropherograms correspond in the genetic tree to (A) the St. Lawrence Island profile and the dotted-line boxes refer to (B) the Chinese rodent profile, (C) the Japanese fox profile, and (D) through (H) the main European profiles. Samples 500, 501 and 502 represent a single isolate maintained in vivo by several passages in Meriones unguiculatus. Sample 116 originating from a Mauritanian camel and sample 539 originating from an Algerian sheep were E. granulosus samples and were included as an out-group control (redrawn from (Knapp et al. Reference Knapp, Bart, Glowatzki, Ito, Gerard, Maillard, Piarroux and Gottstein2007)).
Spatial distribution of various samples of E. multilocularis collected from infected foxes in Europe, and clustered according to geographical peculiarities. Red lozenges represent the position of fox; polygons define a geographically restricted sub-region. The red circle area indicates the historically documented E. multilocularis central endemic focus in Europe, where most humans cases have been recorded in the past five decades (redrawn from Knapp et al. Reference Knapp, Bart, Giraudoux, Glowatzki, Breyer, Raoul, Deplazes, Duscher, Martinek, Dubinsky, Guislain, Cliquet, Romig, Malczewski, Gottstein and Piarroux2009).

Genetic richness (a) and diversity (Inverse Simpson index, b) rarefaction curves for each sub-region (fox as a sampling unit). Swiss: Switzerland, canton of Zurich; NorthAu: North Austria; Swab: Swabian Jura; Bav: Bavaria; Arde: Ardennes; WestCz: West Czech Republic; NorthPol: North Poland; EastSlovPol: East Slovakia and South Poland; CentSlov: Central Slovakia (redrawn from Knapp et al. Reference Knapp, Bart, Giraudoux, Glowatzki, Breyer, Raoul, Deplazes, Duscher, Martinek, Dubinsky, Guislain, Cliquet, Romig, Malczewski, Gottstein and Piarroux2009).

LOCAL SCALE: E. MULTILOCULARIS GENETIC DIVERSITY TRANSMITTED AMONG FOX COMMUNITIES
Several independent studies have documented the value of EmsB to assess the genetic diversities and peculiarities of local E. multilocularis populations within the definitive host. One study was carried out in a mountain area, the Val Pusteria in the North Italy (Casulli et al. Reference Casulli, Bart, Knapp, La Rosa, Dusher, Gottstein, Di Cerbo, Manfredi, Genchi, Piarroux and Pozio2009). When compared to 32 different EmsB profiles described for Central Europe (Knapp et al. Reference Knapp, Bart, Giraudoux, Glowatzki, Breyer, Raoul, Deplazes, Duscher, Martinek, Dubinsky, Guislain, Cliquet, Romig, Malczewski, Gottstein and Piarroux2009), this North Italian region presented only 4 endemic profiles, which suggested the occurrence of a local parasite life cycle in this region independent of South Austria (Knapp et al. Reference Knapp, Bart, Glowatzki, Ito, Gerard, Maillard, Piarroux and Gottstein2007; Casulli et al. Reference Casulli, Bart, Knapp, La Rosa, Dusher, Gottstein, Di Cerbo, Manfredi, Genchi, Piarroux and Pozio2009). The presence of the parasite in the South Alpine region might be explained by the spread of E. multilocularis from the historical core described in the Alpine Arch. As observed in Europe, a founder event probably due to fox dispersion through the Alpine mountain could have permitted the establishment of the E. multilocularis genotypes found in this Italian area, after their proliferation in local foxes (Templeton, Reference Templeton2008). But as these Italian genotypes were not found in neighbouring Austria (Knapp et al. Reference Knapp, Bart, Glowatzki, Ito, Gerard, Maillard, Piarroux and Gottstein2007, Reference Knapp, Bart, Giraudoux, Glowatzki, Breyer, Raoul, Deplazes, Duscher, Martinek, Dubinsky, Guislain, Cliquet, Romig, Malczewski, Gottstein and Piarroux2009) one might suspect other origins of the parasites, e.g. from other areas in Italy. Moreover, one cannot exclude an historic presence of E. multilocularis in the Southern part of Europe, away from the Alps. The recent findings suggest intensive drift of E. multilocularis in Europe for a longer time than was previously thought. Moreover the reports of five cases in Italy more than 100 years ago (Posselt, Reference Posselt1900) confirmed the ancient presence of the parasite in the Southern Alps. But if few exchanges through the Alps occur, the parasite genotype frequency could decrease by a bottleneck phenomenon, due to the mountainous area (Ricklefs and Miller, Reference Ricklefs and Miller2000).
Furthermore, a locally restricted genetic diversity of E. multilocularis was highlighted in a newly recognised endemic region in the Northern part of France (the French Ardennes region). The prevalence of E. multilocularis in this region infected 53% of foxes (Guislain et al. Reference Guislain, Raoul, Giraudoux, Terrier, Froment, Ferte and Poulle2008), and considered as highly endemic. From 140 individual adult worms, collected from 25 foxes, six EmsB profiles were described (Knapp et al. Reference Knapp, Guislain, Bart, Raoul, Gottstein, Giraudoux and Piarroux2008). Genotypically mixed infections were confirmed in foxes, as previously shown in the endemic island of Hokkaido by using the single-locus microsatellite EMms1 (Nakao et al. Reference Nakao, Sako and Ito2003), and EmsB in Europe. A single fox can harbour between 1 to at least 4 different genotypes (Nakao et al. Reference Nakao, Sako and Ito2003; Knapp et al. Reference Knapp, Guislain, Bart, Raoul, Gottstein, Giraudoux and Piarroux2008; Casulli et al. Reference Casulli, Bart, Knapp, La Rosa, Dusher, Gottstein, Di Cerbo, Manfredi, Genchi, Piarroux and Pozio2009), which could depend on the intensity of predation of contaminated rodents and also on the size of the territory investigated by the fox. The simultaneous presence of genotypically different sub-populations of E. multilocularis in fox intestines suggests the possible occurrence of mating events between worms from different populations and yielding of hybrid eggs. Nevertheless the phenomenon was detected only very rarely in collected foxes.
CIRCULATION OF E. MULTILOCULARIS AT A MICRO-LOCAL SCALE
Among our previous sample collection (Knapp et al. Reference Knapp, Bart, Glowatzki, Ito, Gerard, Maillard, Piarroux and Gottstein2007), two panels of naturally infected rodents were collected from fields a few hectares in area in both Switzerland and Alaska were available. The genetic diversity among these related samples was the lowest, and due to these limited genetic differences between samples, these formers were considered to be the most biologically related isolates. One might suspect a common infection of rodents by a unique fox or their contamination after the transmission of a single E. multilocularis strain. These findings inform us of the limits of the genetic discrimination of the EmsB marker and we strongly believe that the EmsB genotyping avoided an over-discrimination even for geographically close related samples (Knapp et al. Reference Knapp, Bart, Glowatzki, Ito, Gerard, Maillard, Piarroux and Gottstein2007).
THE MICROSATELLITE EmsB: A NEW TOOL TO INVESTIGATE THE GENETIC DIVERSITY OF ECHINOCOCCUS GRANULOSUS SENSU LATO
Recently, EmsB was used to characterize 125 samples of E. granulosus s.l. originating from various different host species (sheep, cattle, dromedaries, dogs and human patients) collected in six different countries (Algeria, Mauritania, Romania, Serbia, Brazil and People's Republic of China) (Maillard et al. Reference Maillard, Gottstein, Haag, Ma, Colovic, Benchikh-Elfegoun, Knapp and Piarroux2009). The conventional mitochondrial cox1 and nad1 markers permitted identification of the genotypes G1, G3, G5, G6 and G7, which were clustered into three groups corresponding to the species E. granulosus s.s., E. ortleppi and E. canadensis. The polymorphism exhibited by these markers did not reach the level necessary for the identification of genetic variants within restricted geographical areas. Based on the same samples, EmsB provided a higher genetic discrimination and identified a continental and an intercontinental circulation of the G1 genotypes, the common sheep strain. The trading of the hosts (local and worldwide) and the local migration of (stray) dogs may explain these two types of circulation. Furthermore, the microsatellite EmsB may be potentially useful for taxonomic consideration. The description of mixed G1/G5 profile with EmsB indicated the occurrence of genetic exchanges between distinct E. granulosus s.s. and E. ortleppi populations circulating in Brazil. This result suggests the absence of a strong reproductive barrier between the two species. However these findings encourage further genetic investigations. To summarize, EmsB may be useful for the assessment of the genetic polymorphism of E. granulosus s.l. as well as its taxonomy and details of its spatial distribution. Knapp and co-workers (Reference Knapp2007, Reference Knapp, Bart, Giraudoux, Glowatzki, Breyer, Raoul, Deplazes, Duscher, Martinek, Dubinsky, Guislain, Cliquet, Romig, Malczewski, Gottstein and Piarroux2008) had already shown earlier that this microsatellite enriched a powerful panel of markers to track temporal and spatial transmission of E. multilocularis. In this work, the microsatellite EmsB also exhibited an interesting potential for E. granulosus s.l. because it could be useful for the elaboration of a detailed distribution map of genetic variants and in the determination and tracking of the infection source of CE.
CONCLUSION
In population genetics, with special reference to eco-epidemiology, the development of highly polymorphic tools is necessary to trace infectious organisms in the environment. The parasites E. multilocularis and E. granulosus s.l. appeared as interesting models, because they need two mammalian hosts to perpetuate, with a large range of intermediate hosts. Echinococcus spp. are transported widely by carnivores, the predators of its intermediate hosts, but present a relatively low intraspecific genetic diversity in DNA coding regions. Silent mutations could be analysed to define the evolution of the parasite. EmsB is a novel genetic multi-locus tool and, due to its presence in multi-copies within the Echinococcus genome, offers appropriate methodological sensitivity to trace the genetic variability of E. multilocularis at a hitherto unattainable level. Nevertheless, we have to keep in mind that such research tools provide data which must finally be integrated into a global approach. Numerous parameters have to be taken into account in this analysis, such as geographical data, eco-epidemiology and also human and veterinary health monitoring strategies. These multi-factor studies enabled us to gain a better understanding of the dispersion of an organism in the environment, and the threat it represents to humans. From an eco-epidemiological perspective, one of the crucial future steps to progress molecular-genetic research will be to include human AE and CE patients in this type of topic. The genotyping of parasites transmitted to humans could putatively be used as a complementary tool in health control programmes.
ACKNOWLEDGMENTS
We are very grateful to the different laboratories and institutes where this work was undertaken and for technical help and support: to Prof. Christiane Mougin and Dr Laurent Bermont from the Laboratory of Biochemestry and Cellular Biology, University Hospital, Besançon, France, to Dr Marie-Louise Glowatzki from the Department of Clinical Research, Vetsuisse faculty, Berne, Switzerland. We also thank Karen Haag for constructive comments on our works and Prof. Ito from the Asahikawa Medical College for his support.