





No CrossRef data available.
Article contents
Food environments shape the way mortality influences life-history trajectories
Published online by Cambridge University Press: 11 November 2025
Abstract
The relationship between local extrinsic mortality rates and the timing of life-history milestones can be better understood when examined through food environments rather than by population “types,” like small-scale societies or high-income countries. By mapping observed life-history variation onto food environments, which mediate the fundamental relationship between mortality and fertility, the explanatory value of a 2-tiered model becomes less compelling.
Information
- Type
- Open Peer Commentary
- Information
- Copyright
- © The Author(s), 2025. Published by Cambridge University Press
References
Cetateanu, A. & Jones, A. (2014). Understanding the relationship between food environments, deprivation and childhood overweight and obesity: Evidence from a cross sectional England-wide study. Health & Place 27: 68–76. https://doi.org/10.1016/j.healthplace.2014.01.007
CrossRefGoogle ScholarPubMed
Chisholm, J. (1993). Death, hope, and sex: Life-history theory and the development of reproductive strategies. Current Anthropology 34(1): 1–24.10.1086/204131CrossRefGoogle Scholar
Giskes, K., van Lenthe, F., Avendano-Pabon, M. & Brug, J. (2011). A systematic review of environmental factors and obesogenic dietary intakes among adults: Are we getting closer to understanding obesogenic environments? Obesity Reviews 12(5): e95–e106. https://doi.org/10.1111/j.1467-789X.2010.00769.x
CrossRefGoogle ScholarPubMed
Lee, A., Cardel, M. & Donahoo, W. T. (2000). Social and environmental factors influencing obesity. In Feingold, K. R., Ahmed, S. F., Anawalt, B., Blackman, M. R., Boyce, A., Chrousos, G., Corpas, E., de Herder, W. W., Dhatariya, K., Dungan, K., Hofland, J., Kalra, S., Kaltsas, G., Kapoor, N., Koch, C., Kopp, P., Korbonits, M., Kovacs, C. S., Kuohung, W., …, & Wilson, D. P. (Eds.), Endotext. MDText.com, Inc. http://www.ncbi.nlm.nih.gov/books/NBK278977/
Google Scholar
Pepper, G. V. & Nettle, D. (2014). Perceived extrinsic mortality risk and reported effort in looking after health. Human Nature 25(3): 378–392. https://doi.org/10.1007/s12110-014-9204-5
CrossRefGoogle ScholarPubMed
Pepper, G. V. & Nettle, D. (2017). The behavioural constellation of deprivation: Causes and consequences. The Behavioral and Brain Sciences 40: e314. https://doi.org/10.1017/S0140525X1600234X
CrossRefGoogle ScholarPubMed
Sheppard, P., Garcia, J. R. & Sear, R. (2015). Childhood family disruption and adult height: Is there a mediating role of puberty? Evolution, Medicine, and Public Health 2015(1): 332–342.10.1093/emph/eov028CrossRefGoogle Scholar
Sheppard, P., Pearce, M. & Sear, R. (2016). How does childhood socioeconomic hardship affect reproductive strategy? Pathways of development. American Journal of Human Biology 28(3): 356–363.10.1002/ajhb.22793CrossRefGoogle ScholarPubMed
Sheppard, P. & Van Winkle, Z. (2020). Using sequence analysis to test if human life histories are coherent strategies. Evolutionary Human Sciences 2: e39. https://doi.org/10.1017/ehs.2020.38
CrossRefGoogle ScholarPubMed
Stearns, S., Ackermann, M., Doebeli, M. & Kaiser, M. (2000). Experimental evolution of aging, growth, and reproduction in fruitflies. Proceedings of the National Academy of Sciences of the United States of America 97(7): 3309–3313. https://doi.org/10.1073/pnas.060289597
CrossRefGoogle ScholarPubMed
Stearns, S. C. & Rodrigues, A. M. M. (2020). On the use of “life history theory” in evolutionary psychology. Evolution and Human Behavior 41(6): 474–485. https://doi.org/10.1016/j.evolhumbehav.2020.02.001
CrossRefGoogle Scholar
Ulijaszek, S. (2024). Understanding Obesity (New edition). Cambridge: Cambridge University Press.10.1017/9781009218184CrossRefGoogle Scholar
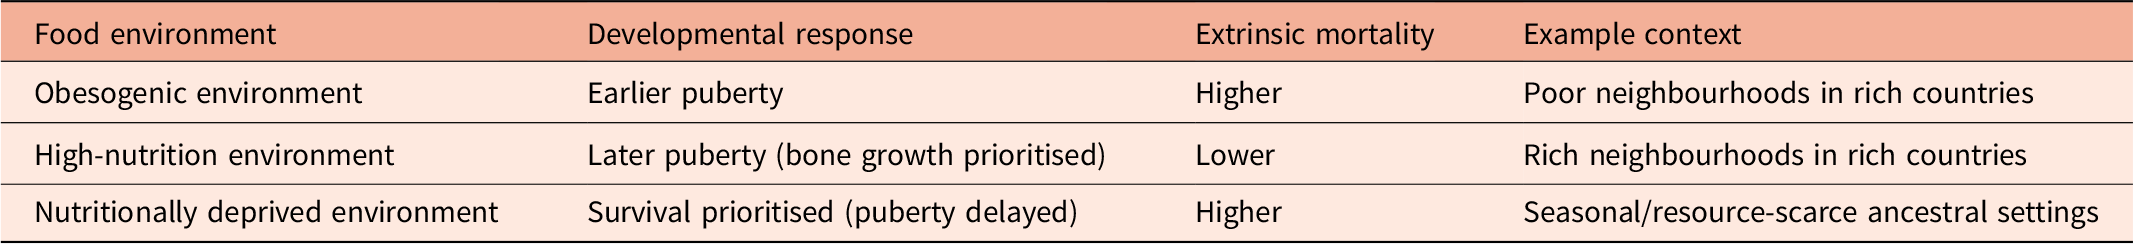
Table 1. Expected responses to mortality in different food environments
Target article
Related commentaries (29)
Density slows, while pathogens and disasters accelerate life history within populations
Hierarchical response models: new perspectives on development
The mortality-fertility relationship from the economic demography perspective
 You have
Access
It is refreshing to see more nuanced approaches to how life-history models can be applied to humans. Ellis, Reid, and Kramer compose an intricate 2-tier model to better understand the global variation we see in sexual maturation and reproductive timings and how they are linked to extrinsic mortality rates. It might also be helpful to think about this in relation to food environments rather than by “types” of society (small-scale, industrialised, etc.), which assumes that mortality rates and food security are constant within each context. In small-scale societies, local extrinsic mortality rates change over time, and food security changes with the season or due to natural fluctuations. In industrialised countries, mortality rates and food availability vary by socioeconomic strata. Focusing on changing food environments produces a simpler explanation for thinking about how local mortality rates affect puberty, growth, and fertility.
In wealthy countries, children who live in poverty often inhabit obesogenic environments with an overabundance of highly calorific, ultra-processed foods that are low on nutritional value (Cetateanu & Jones, Reference Cetateanu and Jones2014; Giskes et al., Reference Giskes, van Lenthe, Avendano-Pabon and Brug2011; Lee et al., Reference Lee, Cardel, Donahoo, Feingold, Ahmed, Anawalt, Blackman, Boyce, Chrousos, Corpas, de Herder, Dhatariya, Dungan, Hofland, Kalra, Kaltsas, Kapoor, Koch, Kopp, Korbonits, Kovacs, Kuohung and Wilson2000; Ulijaszek, Reference Ulijaszek2024). This promotes the production of adipose tissue and early pubertal maturity, especially for girls (Sheppard et al., Reference Sheppard, Garcia and Sear2015). In contrast, girls in wealthier neighbourhoods eat more nutrient-rich high-fibre diets, which promote skeletal growth and later pubertal maturity, as characterised by the growth-reproduction life-history trade-off. In small-scale societies that inhabit environments that are closer to what we imagine our evolutionary past to have been like, food would be of relatively higher nutritional value but less abundant than what we see in contemporary high-income countries. Access to nutritious food is expected to promote skeletal growth and slower pubertal development, but at the same time, those groups who struggle to get enough food at all will slow bone growth and pubertal development due to the adaptive strategy to simply stay alive, i.e. the trade-off between survival and growth/maintenance. This is why, overall, age at puberty is later, on average, in resource-stressed settings compared to in high-income countries, but the variation observed within each setting can be explained by differential types of nutrition (Sheppard & Van Winkle, Reference Sheppard and Van Winkle2020; Stearns & Rodrigues, Reference Stearns and Rodrigues2020). “Energetics” is therefore too simple a term; what matters is the type of energy – simply calorific or high nutritional quality – leading to either adiposity or skeletal growth. Table 1 summarises this argument.
Expected responses to mortality in different food environments
Among disadvantaged populations in wealthy countries, the life-history prediction is that higher extrinsic mortality rates, characteristic of deprived neighbourhoods, promote faster sexual maturity and higher fertility, with the mechanism being access to high-calorie, low-nutrition food. In high-income countries, there is a suite of related risks that come with poverty; father absence, higher crime rates, substance abuse, etc. (Pepper & Nettle, Reference Pepper and Nettle2014, Reference Pepper and Nettle2017; Sheppard et al., Reference Sheppard, Pearce and Sear2016) that all contribute to increased perceived extrinsic mortality risk, which is associated with early sexual maturation and higher birth rates. These stressors are embodied via various hormonal reactions such as elevated cortisol and reduced androgens, which affect the rate of development (albeit differently for boys and girls) (Sheppard et al., Reference Sheppard, Garcia and Sear2015). The point is that this is allowed to happen because the food is there, if it weren’t – if these neighbourhoods were food barren like in some very harsh ancestral conditions – puberty would be later in favour of survival.
Thinking about our evolutionary past, when subjected to high rates of ambient extrinsic mortality, we would still expect to see faster maturation and more births (not necessarily surviving), but only if there is enough food to do so; if there is insufficient food, it is better to prioritise survival. If mortality is high and food is plentiful, then everything speeds up to offset the risk of dying (Chisholm, Reference Chisholm1993; Stearns et al., Reference Stearns, Ackermann, Doebeli and Kaiser2000). When mortality is low and food is scarce, things slow down, and when mortality is low and food is plentiful, then things are neither fast nor slow because trade-offs are strongest when conditions are harsh.
While the 2-tiered model offers a valuable synthesis of how mortality and energetics influence development and fertility, its core insights may appear more novel than they are. Researchers working in this space generally recognise that energetics and mortality exposure are context-dependent and interact in complex ways. What this model does well is highlight the need to disentangle different pathways, but it may also overcomplicate what can be more parsimoniously understood by situating mortality cues within their nutritional setting rather than by population type.
Funding statement
This work is not funded.
Competing interests
I declare no competing interests.