Refine search
Actions for selected content:
113 results
Role of dimension and geometry: non-uniqueness in the pseudo-one-dimensional limit for Turing patterns on parallelograms
- Part of
-
- Journal:
- European Journal of Applied Mathematics , First View
- Published online by Cambridge University Press:
- 29 September 2026, pp. 1-20
-
- Article
-
- You have access
- Open access
- HTML
- Export citation
The lingering phenomenon and pattern formation in a nonlocal population model with cognitive map
- Part of
-
- Journal:
- European Journal of Applied Mathematics , First View
- Published online by Cambridge University Press:
- 21 September 2026, pp. 1-24
-
- Article
-
- You have access
- Open access
- HTML
- Export citation
The effect of local ventilation on a spatiotemporal model of airborne disease transmission in indoor spaces
- Part of
-
- Journal:
- European Journal of Applied Mathematics , First View
- Published online by Cambridge University Press:
- 15 July 2026, pp. 1-18
-
- Article
-
- You have access
- Open access
- HTML
- Export citation
-
We incorporate local ventilation effects into a spatially dependent generalisation of the Wells–Riley model for airborne disease transmission and consider a room in which an air purifier supplements the ventilation provided by a poorly functioning air-conditioning (AC) unit. Aerosol production and removal through ventilation, biological deactivation and gravitational settling as well as transport around a recirculating AC flow and global turbulent mixing are modelled using an advection–diffusion–reaction equation. This local ventilation model is compared with a global ventilation model, where all ventilation is treated as a global sink. We undertake this comparison for a weak purifier (clean air delivery rate of 140 m
 $^3$h
 $^{-1}$) and a strong purifier (clean air delivery rate of 1,000 m
 $^3$h
 $^{-1}$). For each purifier, we determine a total effective air exchange rate and compare against the global model with equivalent ventilation. We find that, as expected, the purifier removes fewer aerosols when the distance between the infectious person and the purifier is increased, resulting in a greater average aerosol concentration in the room. Moreover, the concentration is generally lowest when the infectious person is upstream of the purifier, located in regions where the airflow streamlines are directed into the purifier. For these infectious source locations, the global ventilation model significantly overestimates the concentration throughout the room. For infectious sources outside of these regions, there is generally good agreement between the models, particularly for the weak purifier. We also studied, for a fixed distance from the purifier, how the infection risk to a susceptible person varies as the infectious person changes location. A susceptible person faces the highest infection risk when they are directly downstream of the infectious person, where the aerosol concentration is the highest. There is better agreement between local and global ventilation models for the weak purifier than for the strong purifier since the weak purifier has less impact on the airflow in the room.


Spatial dynamics of a partially degenerate reaction–diffusion system with pair formation
- Part of
-
- Journal:
- Canadian Journal of Mathematics , First View
- Published online by Cambridge University Press:
- 07 July 2026, pp. 1-28
-
- Article
-
- You have access
- HTML
- Export citation
Cognitive diffusion of susceptibles driven by new infection cases in SIS epidemic models: frequency-dependent incidence
- Part of
-
- Journal:
- European Journal of Applied Mathematics , First View
- Published online by Cambridge University Press:
- 10 June 2026, pp. 1-29
-
- Article
-
- You have access
- Open access
- HTML
- Export citation
On the dynamics of a diffusive SEIRS epidemic model
- Part of
-
- Journal:
- European Journal of Applied Mathematics / Volume 37 / Issue 6 / December 2026
- Published online by Cambridge University Press:
- 13 April 2026, pp. 1420-1464
-
- Article
-
- You have access
- Open access
- HTML
- Export citation
-
This work investigates the dynamics of positive classical solutions to a diffusive susceptible-exposed-infected-recovered-susceptible epidemic model with a mass-action incidence mechanism in spatially heterogeneous environments. Under minimal assumptions on the initial data, the global existence of classical solutions is established. Moreover, the eventual boundedness of these solutions is proved when either the spatial domain has dimension five or lower or the susceptible and exposed subpopulations share the same diffusion rate. Next, we define the basic reproduction number,
 $\mathcal{R}_0$, and demonstrate that the disease-free equilibrium is globally stable when
 $\mathcal{R}_0$ is sufficiently small. However, due to the complex interaction between population movement and spatial variation in transmission rates, we find that the disease may persist even when
 $\mathcal{R}_0$ is slightly less than one. In such cases, we show that the system admits at least two endemic equilibrium (EE) solutions, an outcome not observed under the frequency-dependent incidence mechanism. These results highlight the significant influence of the transmission mechanism on disease dynamics. Furthermore, we examine the spatial profiles of the EE solutions when diffusion rates are small. Our analysis suggests that limiting the movement of the susceptible population can significantly reduce disease prevalence, provided that the total population remains below a specific threshold. In contrast, restricting the movement of the infected, exposed, or recovered populations alone may not eradicate the disease. Overall, our findings provide important insights into the spatial dynamics of infectious diseases and may offer guidance for developing and implementing effective containment strategies.


Threshold dynamics of a time-periodic SIS model with anomalous diffusion in heterogeneous environments
- Part of
-
- Journal:
- Proceedings of the Royal Society of Edinburgh. Section A: Mathematics , First View
- Published online by Cambridge University Press:
- 24 February 2026, pp. 1-28
-
- Article
-
- You have access
- HTML
- Export citation
Periodic dynamics in a time-switching advection-diffusion model for competing Aedes mosquitoes
- Part of
-
- Journal:
- European Journal of Applied Mathematics / Volume 37 / Issue 5 / October 2026
- Published online by Cambridge University Press:
- 16 February 2026, pp. 1292-1312
-
- Article
-
- You have access
- Open access
- HTML
- Export citation
Competition of small targets in planar domains: from Dirichlet to Robin and Steklov boundary condition
- Part of
-
- Journal:
- European Journal of Applied Mathematics / Volume 37 / Issue 5 / October 2026
- Published online by Cambridge University Press:
- 12 January 2026, pp. 1244-1291
-
- Article
-
- You have access
- Open access
- HTML
- Export citation
Propagation dynamics of time-dependent reaction-diffusion equations under climate change in an infinite cylinder
- Part of
-
- Journal:
- European Journal of Applied Mathematics / Volume 37 / Issue 5 / October 2026
- Published online by Cambridge University Press:
- 19 December 2025, pp. 1200-1221
-
- Article
-
- You have access
- Open access
- HTML
- Export citation
-
In this paper, we consider a reaction-diffusion equation that models the time-almost periodic response to climate change within a straight, infinite cylindrical domain. The shifting edge of the habitat is characterised by a time-almost periodic function, reflecting the varying pace of environmental changes. Note that the principal spectral theory is an important role to study the dynamics of reaction-diffusion equations in time heterogeneous environment. Initially, for time-almost periodic parabolic equations in finite cylindrical domains, we develop the principal spectral theory of such equations with mixed Dirichlet–Neumann boundary conditions. Subsequently, we demonstrate that the approximate principal Lyapunov exponent serves as a definitive threshold for species persistence versus extinction. Then, the existence, exponential decay and stability of the forced wave solutions
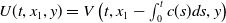 $U(t,x_{1},y)=V\left (t,x_{1}-\int ^{t}_{0}c(s)ds,y\right )$ are established. Additionally, we analyse how fluctuations in the shifting speed affect the approximate top Lyapunov exponent.
Impact of birth pulse and environment shift on population survival and propagation
- Part of
-
- Journal:
- Canadian Journal of Mathematics , First View
- Published online by Cambridge University Press:
- 17 October 2025, pp. 1-27
-
- Article
-
- You have access
- HTML
- Export citation
Global dynamics of a degenerate reaction-diffusion cholera model with phage-bacteria interaction in a heterogeneous environment
- Part of
-
- Journal:
- European Journal of Applied Mathematics / Volume 37 / Issue 4 / August 2026
- Published online by Cambridge University Press:
- 22 September 2025, pp. 1002-1033
-
- Article
-
- You have access
- Open access
- HTML
- Export citation
-
To investigate multiple effects of the interaction between V. cholerae and phage on cholera transmission, we propose a degenerate reaction-diffusion model with different dispersal rates, which incorporates a short-lived hyperinfectious (HI vibrios) state of V. cholerae and lower-infectious (LI vibrios) state of V. cholerae. Our main purpose is to investigate the existence and stability analysis of multi-class boundary steady states, which is much more complicated and challenging than the case when the boundary steady state is unique. In a spatially heterogeneous case, the basic reproduction number
 $\mathscr{R}_{0}$ is defined as the spectral radius of the sum of two linear operators associated with HI vibrios infection and LI vibrios infection. If
 $\mathscr{R}_{0}\leq 1$, the disease-free steady state is globally asymptotically stable. If
 $\mathscr{R}_{0}\gt 1$, the uniform persistence of phage-free model, as well as the existence of the phage-free steady state, are established. In a spatially homogeneous case, when
 $\ \;\widetilde{\!\!\!\mathscr{R}}_{0}\gt 1$, the global asymptotic stability of phage-free steady state and the uniform persistence of the phage-present model are discussed under some additional conditions. The mathematical approach here has wide applications in degenerate Partial Differential Equations.


Existence-uniqueness theory and small-data decay for a reaction-diffusion model of wildfire spread
- Part of
-
- Journal:
- Canadian Mathematical Bulletin / Volume 68 / Issue 4 / December 2025
- Published online by Cambridge University Press:
- 08 July 2025, pp. 1347-1358
- Print publication:
- December 2025
-
- Article
-
- You have access
- HTML
- Export citation
-
I examine some analytical properties of a nonlinear reaction-diffusion system that has been used to model the propagation of a wildfire. I establish global-in-time existence and uniqueness of bounded mild solutions to the Cauchy problem for this system given bounded initial data. In particular, this shows that the model does not allow for thermal blow-up. If the initial temperature and fuel density also satisfy certain integrability conditions, the spatial
 $L^2$-norms of these global solutions are uniformly bounded in time. Additionally, I use a bootstrap argument to show that small initial temperatures give rise to solutions that decay to zero as time goes to infinity, proving the existence of initial states that do not develop into traveling combustion waves.

A free boundary problem of competition-diffusion system with Dirichlet boundary condition
- Part of
-
- Journal:
- Canadian Mathematical Bulletin / Volume 69 / Issue 1 / March 2026
- Published online by Cambridge University Press:
- 07 July 2025, pp. 1-20
- Print publication:
- March 2026
-
- Article
-
- You have access
- HTML
- Export citation
-
In this article, we investigate a free boundary problem for the Lotka–Volterra model consisting of an invasive species with density u and a native species with density v in one dimension. We assume that v undergoes diffusion and growth in
 $[0,+\infty )$, and u invades into the environment with spreading front
 $x=h(t)$ satisfying free boundary condition
 $h'(t)=-u_x(t,h(t))-\alpha $ for some decay rate
 $\alpha>0$, this is caused by the bad environment at the boundary. When u is an inferior competitor,
 $u(t,x)$ and
 $h(t)$ tend to 0 within a finite time, while another specie
 $v(t,x)$ tends to a stationary
 $\Lambda (x)$ defined on the half-line. When u is a superior competitor, we have a trichotomy result: spreading of u and vanishing of v (i.e., as
 $t \to +\infty $,
 $h(t)$ goes to
 $+\infty $ and
 $(u,v)\to (\Lambda ,0)$); the transition case (i.e., as
 $t \to +\infty $,
 $(u,v)\to (w_\alpha , \eta _\alpha )$,
 $h(t)$ tends to a finite point); vanishing of u and spreading of v (i.e.,
 $u(t,x)$ and
 $h(t)$ tends to 0 within a finite time,
 $v(t,x)$ converges to
 $\Lambda (x)$). Additionally, we show that this trichotomy result depends on the initial data
 $u(0,x)$.


The evolution problem for the 1D nonlocal Fisher-KPP equation with a top hat kernel. Part 2. The initial-boundary value problem on a finite domain
- Part of
-
- Journal:
- European Journal of Applied Mathematics / Volume 37 / Issue 2 / April 2026
- Published online by Cambridge University Press:
- 04 July 2025, pp. 520-550
-
- Article
-
- You have access
- Open access
- HTML
- Export citation
-
In the second part of this series of papers, we address the same evolution problem that was considered in part 1 (see [16]), namely the nonlocal Fisher-KPP equation in one spatial dimension,
where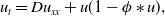 \begin{equation*} u_t = D u_{xx} + u(1-\phi *u), \end{equation*}
 $\phi *u$ is a spatial convolution with the top hat kernel,
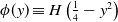 $\phi (y) \equiv H\left (\frac {1}{4}-y^2\right )$, except that now we modify this to an associated initial-boundary value problem on the finite spatial interval
 $[0,a]$ rather than the whole real line. Boundary conditions are required at the end points of the interval, and we address the situations when these are of either Dirichlet or Neumann type. This model is a natural extension of the classical Fisher-KPP model, with the introduction of the simplest possible nonlocal effect into the saturation term. Nonlocal reaction-diffusion models arise naturally in a variety of (frequently biological or ecological) contexts, and as such it is of fundamental interest to examine their properties in detail, and to compare and contrast these with the well known properties of the classical Fisher-KPP model.


DELAYED HOPF BIFURCATIONS IN REACTION–DIFFUSION SYSTEMS IN TWO SPACE DIMENSIONS
- Part of
-
- Journal:
- The ANZIAM Journal / Volume 67 / 2025
- Published online by Cambridge University Press:
- 13 May 2025, e19
-
- Article
-
- You have access
- Open access
- HTML
- Export citation
Pattern formation with jump discontinuity in a predator–prey model with Holling-II functional response
- Part of
-
- Journal:
- European Journal of Applied Mathematics / Volume 36 / Issue 6 / December 2025
- Published online by Cambridge University Press:
- 11 April 2025, pp. 1160-1182
-
- Article
-
- You have access
- Open access
- HTML
- Export citation
Spatio-temporal dynamics of a lattice prey–predator system with non-local diffusion in a periodic habitat
- Part of
-
- Journal:
- Proceedings of the Royal Society of Edinburgh. Section A: Mathematics , First View
- Published online by Cambridge University Press:
- 31 March 2025, pp. 1-43
-
- Article
-
- You have access
- HTML
- Export citation
Impact of prey-taxis on a harvested intraguild predation predator–prey model
- Part of
-
- Journal:
- European Journal of Applied Mathematics / Volume 36 / Issue 6 / December 2025
- Published online by Cambridge University Press:
- 10 March 2025, pp. 1183-1220
-
- Article
-
- You have access
- Open access
- HTML
- Export citation
A critical non-homogeneous heat equation with weighted source
- Part of
-
- Journal:
- European Journal of Applied Mathematics / Volume 36 / Issue 6 / December 2025
- Published online by Cambridge University Press:
- 06 March 2025, pp. 1148-1159
-
- Article
-
- You have access
- Open access
- HTML
- Export citation
-
Some qualitative properties of radially symmetric solutions to the non-homogeneous heat equation with critical density and weighted source
are obtained, in the range of exponents \begin{align*} |x|^{-2}\partial _tu=\Delta u+|x|^{\sigma }u^p, \quad (x,t)\in {\mathbb {R}}^N\times (0,T), \end{align*}
 $p\gt 1$,
 $\sigma \ge -2$. More precisely, we establish conditions fulfilled by the initial data in order for the solutions to either blow-up in finite time or decay to zero as
 $t\to \infty$ and, in the latter case, we also deduce decay rates and large time behavior. In the limiting case
 $\sigma =-2$, we prove the existence of non-trivial, non-negative solutions, in stark contrast to the homogeneous case. A transformation to a generalized Fisher–KPP equation is derived and employed in order to deduce these properties.


